Metabolism & Nutrition
Every second you are alive, thousands of chemical reactions are running inside your cells — some building, some breaking down, all of them handling energy. That entire web of reactions is metabolism, and this chapter is where the food on your plate finally meets the machinery of your cells. You will follow a molecule of glucose as it is dismantled to power an ATP, watch your body flip between storing fuel after a meal and spending it between meals, and learn what the six classes of nutrients actually do once they are inside you. By the end, the deceptively simple question — why do we eat? — will have a precise, satisfying answer.
By the end of this chapter you can
- Define metabolism and distinguish anabolism from catabolism by their direction and their handling of energy.
- Explain how ATP stores and delivers energy, and how catabolism is coupled to anabolism.
- Trace glucose through the four steps of cellular respiration and account for the ATP produced at each stage.
- Explain why oxygen is required for aerobic respiration and what the cell does when it runs short.
- Contrast the absorptive and postabsorptive metabolic states and the roles of insulin and glucagon.
- Name the six classes of nutrients, state which yield energy, and give each one's caloric value.
- Separate the fat-soluble from the water-soluble vitamins and predict which are stored and which must be eaten regularly.
- Describe energy balance and the three parts of total energy expenditure.
Section 1Anabolism & catabolism
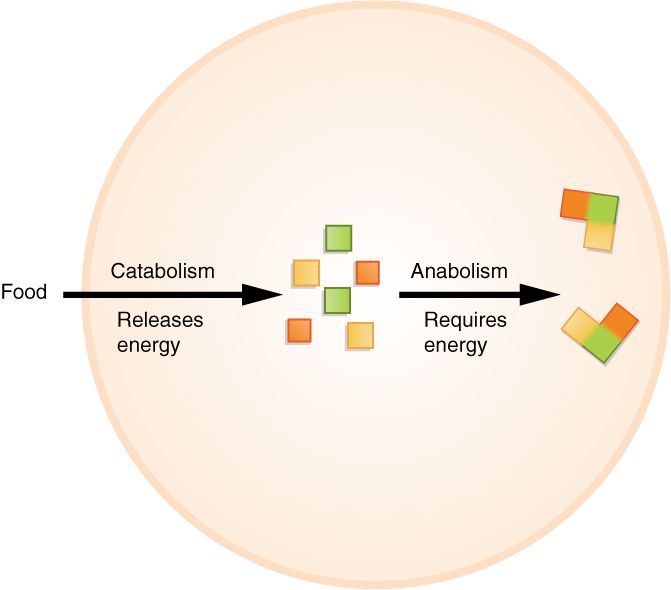
One word for every reaction
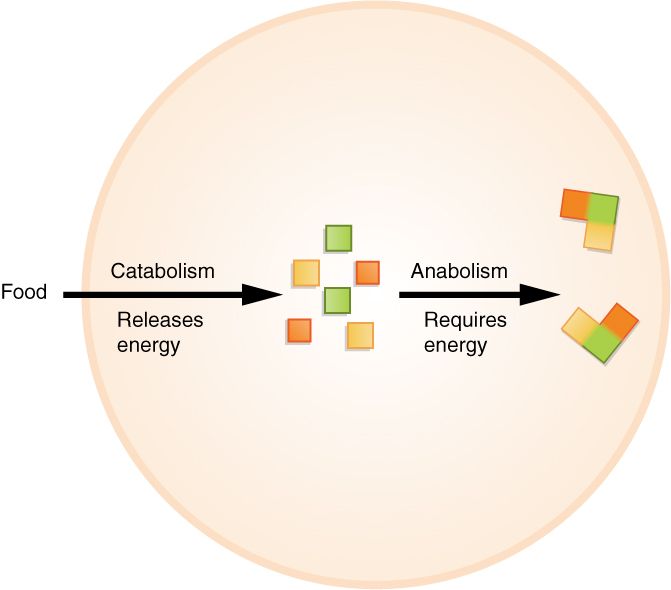
Metabolism is the sum of every chemical reaction in the body — and there are staggering numbers of them running at once. To make that ocean learnable, we sort every reaction into one of two directions. Anabolism is the building direction: small molecules are joined into larger ones, usually by dehydration synthesis (removing a water molecule to form a bond). Amino acids become proteins, glucose units become glycogen, fatty acids and glycerol become fat. Building costs energy, so anabolic reactions are endergonic — they must be paid for. Catabolism is the breaking-down direction: large molecules are split into smaller ones, usually by hydrolysis (adding water to break a bond). Catabolism releases the energy that was locked in those chemical bonds, so these reactions are exergonic — they pay out. The two directions are not separate businesses; the energy released by catabolism is precisely what funds anabolism.
ATP: the cell's rechargeable battery
The body does not spend food energy directly. Instead it converts that energy into a single, universal currency — ATP (adenosine triphosphate). ATP carries its energy in the bonds between its three phosphate groups. Snap off the last phosphate and you get ADP plus a free phosphate plus a burst of usable energy; the cell uses that burst to power muscle contraction, nerve signaling, and anabolic building. Catabolism then recharges the battery by bolting the phosphate back on, turning ADP back into ATP. This constant charge-and-discharge is called energy coupling: an exergonic reaction (breaking a bond) is linked to an endergonic one (doing work) so the energy is handed off rather than lost as heat. You cycle your entire body weight in ATP roughly every day — not because you store that much, but because each molecule is recharged thousands of times.
Following the electrons
Many metabolic reactions are oxidation-reduction (redox) reactions, in which electrons are transferred from one molecule to another. A molecule that loses electrons is oxidized; one that gains them is reduced. This matters because electrons carry energy, and the cell moves them around using shuttle molecules called electron carriers — chiefly NAD⁺ and FAD. When these carriers pick up electrons (becoming NADH and FADH₂), they are essentially loading up on energy to deliver later. Hold onto that idea; in the next section those loaded carriers become the key to making most of your ATP.
| Feature | Anabolism | Catabolism |
|---|---|---|
| Direction | Builds large molecules from small | Breaks large molecules into small |
| Reaction type | Dehydration synthesis | Hydrolysis |
| Energy | Requires energy (endergonic); uses ATP | Releases energy (exergonic); makes ATP |
| Example | Amino acids → protein; glucose → glycogen | Protein → amino acids; glycogen → glucose |
Switch between the building and breaking directions in the interactive below.
- Metabolism = all body reactions; anabolism builds (endergonic, uses ATP), catabolism breaks down (exergonic, makes ATP).
- ATP is the cell's energy currency — it discharges to ADP + phosphate to do work, and catabolism recharges it.
- Energy coupling links energy-releasing reactions to energy-requiring ones so the energy is used, not wasted.
- Electron carriers NAD⁺ and FAD shuttle energy-rich electrons from catabolism to ATP production.
Section 2Cellular respiration
Burning glucose, carefully
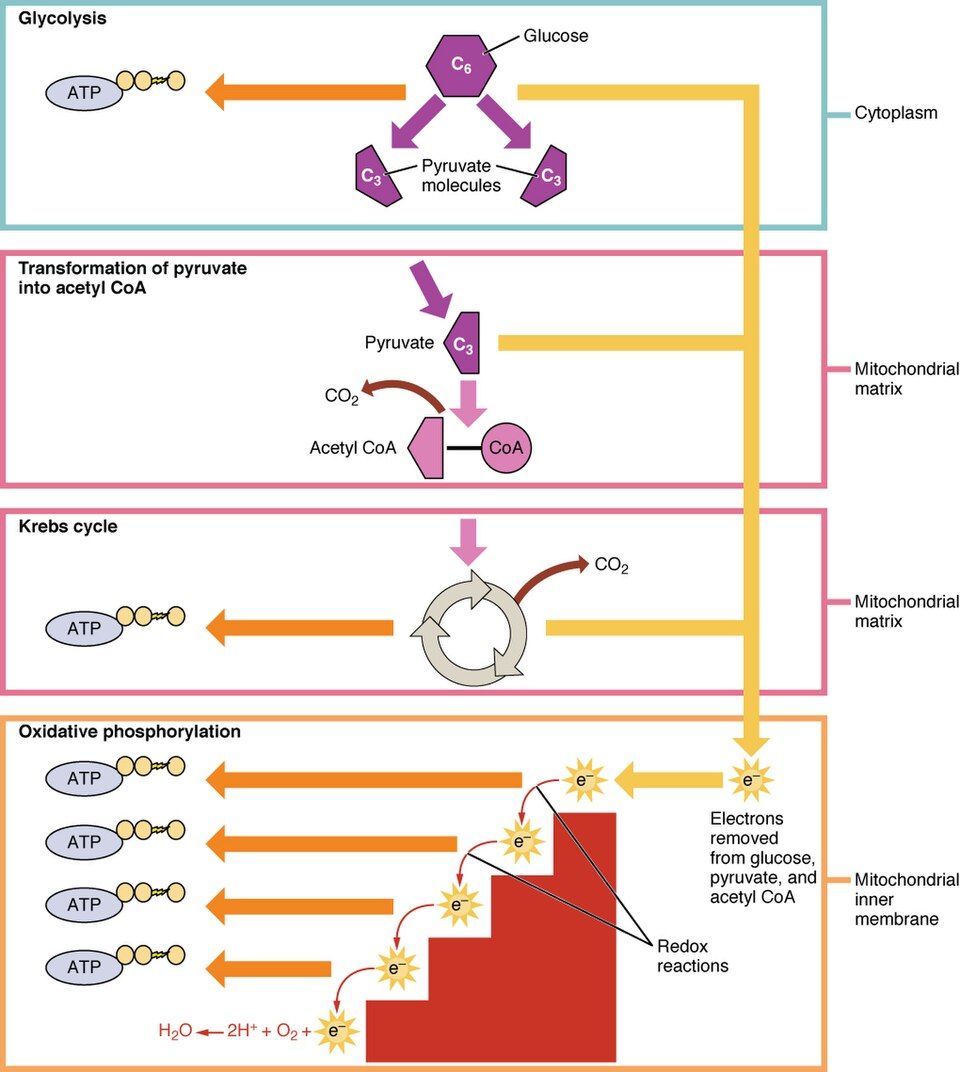
Cellular respiration is the controlled catabolism of glucose to make ATP. It is a kind of slow, safe burning — instead of releasing all of glucose's energy at once as a destructive flash, the cell strips it away in small steps, capturing the energy in ATP as it goes. The whole process happens in four stages across two locations: the first stage in the cytoplasm, the last three inside the mitochondrion. When enough oxygen is present, a single glucose molecule can yield up to roughly 30 to 32 ATP. Follow it stage by stage.
The four stages
1. Glycolysis happens in the cytoplasm and needs no oxygen. One six-carbon glucose is split into two three-carbon pyruvate molecules. The cell spends two ATP to start the process and harvests four, for a net gain of 2 ATP, plus 2 NADH. 2. Pyruvate oxidation (the transition reaction) moves each pyruvate into the mitochondrial matrix, snips off a carbon as CO₂, and attaches the remainder to a carrier to form acetyl CoA, making more NADH. 3. The citric acid cycle (Krebs cycle), also in the matrix, feeds acetyl CoA around a loop that releases the rest of the carbons as CO₂, yields a little more ATP directly, and — most importantly — loads up many molecules of NADH and FADH₂. 4. Oxidative phosphorylation on the inner mitochondrial membrane is where the real payoff comes. The loaded carriers drop their electrons into the electron transport chain, which uses that energy to pump H⁺ ions and build a gradient; the ions then rush back through an enzyme that spins like a turbine, snapping phosphates onto ADP. This step alone makes the large majority of the ATP.
| Stage | Location | Needs O₂? | Main products |
|---|---|---|---|
| Glycolysis | Cytoplasm | No | 2 pyruvate, net 2 ATP, 2 NADH |
| Pyruvate oxidation | Mitochondrial matrix | Yes (aerobic) | Acetyl CoA, CO₂, NADH |
| Citric acid cycle | Mitochondrial matrix | Yes (aerobic) | CO₂, 2 ATP, NADH, FADH₂ |
| Oxidative phosphorylation | Inner mitochondrial membrane | Yes | ~26–28 ATP, H₂O |
Why oxygen, and what happens without it
Here is the punchline of the whole process: oxygen is the final electron acceptor. At the very end of the electron transport chain, the spent electrons and some H⁺ ions are handed to O₂, forming H₂O (the water you make from breathing). If no oxygen is waiting there to accept them, the chain backs up like a clogged drain, the carriers stay loaded, and stages 2 through 4 grind to a halt. When that happens, the cell falls back on anaerobic fermentation: it keeps glycolysis limping along by converting pyruvate to lactic acid, which regenerates the NAD⁺ glycolysis needs. This buys a fast trickle of 2 ATP with no oxygen — useful for a sprinting muscle — but it is wildly inefficient and the lactic acid builds up, which is part of why hard exercise burns.
Step through all four stages and watch the ATP add up in the interactive.
- Cellular respiration = controlled glucose catabolism yielding up to ~30–32 ATP.
- Four stages: glycolysis (cytoplasm) → pyruvate oxidation → citric acid cycle (matrix) → oxidative phosphorylation (inner membrane).
- Oxidative phosphorylation makes most of the ATP, and O₂ is the final electron acceptor, forming water.
- Without oxygen, cells use anaerobic fermentation — only 2 ATP per glucose, with lactic acid as the byproduct.
Section 3Metabolic states: fed vs fasting
Two modes: store or spend
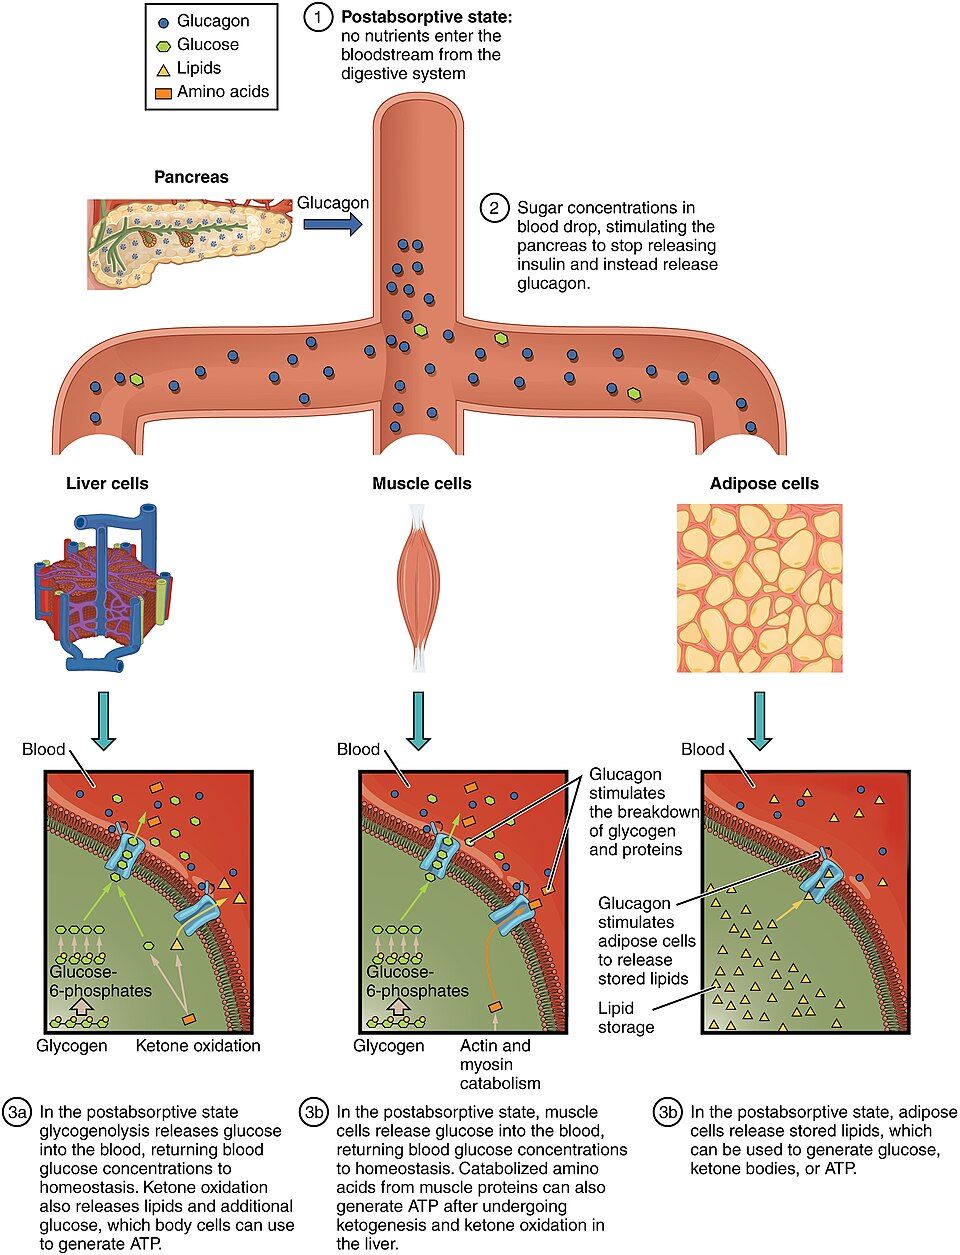
Your fuel supply is not constant — it arrives in bursts at mealtimes and then dwindles for hours afterward. To cope, the body runs in two distinct metabolic states. The absorptive (fed) state is the few hours after a meal, when nutrients are pouring in from the gut and blood glucose rises. The task now is to store the surplus: extra glucose is packed into glycogen (glycogenesis) and fat (lipogenesis), and amino acids build protein. The postabsorptive (fasting) state takes over once absorption is done — overnight, between meals, or during a fast. Now the task flips to releasing stored fuel to keep blood glucose steady: glycogen is broken back to glucose (glycogenolysis), fat is broken down (lipolysis), and the liver even manufactures brand-new glucose from non-carbohydrate sources like amino acids (gluconeogenesis).
Two hormones run the switch
The state you are in is set mainly by two opposing pancreatic hormones. Insulin is the storage hormone; it rises after a meal, drives glucose into cells, and turns on all the building pathways. Glucagon is the mobilizing hormone; it rises during fasting and turns on the releasing pathways. Think of them as a seesaw: insulin high means store, glucagon high means spend. One organ is the hub for all of it — the liver, which stores glycogen after meals and pumps out glucose between them, keeping blood sugar within its narrow homeostatic range around the clock.
Protecting the brain
Why go to all this trouble? Because the brain runs almost exclusively on glucose and cannot store its own fuel, so blood glucose must never crash. During a long fast the body practices glucose sparing: most tissues switch to burning fatty acids, leaving the scarce glucose for the brain. In prolonged starvation the liver converts fat into ketone bodies, an alternative fuel the brain can partly use — a clever adaptation, though a heavy buildup of these acidic ketones can dangerously lower blood pH.
| Feature | Absorptive (fed) | Postabsorptive (fasting) |
|---|---|---|
| When | Hours after a meal | Between meals, overnight, fasting |
| Goal | Store surplus fuel | Release stored fuel |
| Dominant hormone | Insulin | Glucagon |
| Key processes | Glycogenesis, lipogenesis, protein synthesis | Glycogenolysis, lipolysis, gluconeogenesis, ketogenesis |
| Blood glucose trend | Rising → stored | Falling → defended |
Flip between the fed and fasting states in the interactive below.
- The absorptive state stores surplus fuel (glycogenesis, lipogenesis); the postabsorptive state releases it (glycogenolysis, gluconeogenesis, lipolysis).
- Insulin drives storage; glucagon drives mobilization — a seesaw centered on the liver.
- The brain depends on glucose, so fasting metabolism defends blood sugar via glucose sparing and, if prolonged, ketone bodies.
Section 4The six nutrient classes
Three that fuel you, three that don't
Everything worth eating falls into six classes of nutrients. Three of them supply usable energy and are eaten in large amounts — the macronutrients: carbohydrates, lipids (fats), and proteins. The other three yield no energy at all but are absolutely required in smaller amounts — vitamins, minerals, and water. "No energy" does not mean "optional": you would die without water or without trace minerals long before you starved. Each class has a job. Carbohydrates are the body's preferred quick fuel. Lipids are the densest energy store and build every cell membrane. Proteins are mainly structural and functional — enzymes, muscle, antibodies — and are burned for energy only as a last resort.
How much energy is in food?
The energy in food is measured in kilocalories (written "Calories" with a capital C on food labels). Only the three macronutrients carry calories, and they are not equal. Carbohydrate and protein each release about 4 kcal per gram; fat packs more than twice that at about 9 kcal per gram, which is exactly why fatty foods are so calorie-dense and why fat is the body's chosen long-term energy store. Alcohol, though not a nutrient, also carries energy at about 7 kcal per gram.
Essential nutrients: the ones you must eat
An essential nutrient is one your body cannot make (or cannot make in sufficient amounts), so it must come from the diet. These include roughly nine essential amino acids, a couple of essential fatty acids, and all the vitamins and minerals. This is why protein quality matters: a complete protein (from meat, eggs, dairy, soy) supplies all the essential amino acids, while most single plant foods are incomplete — but combining complementary plants, such as beans with rice, covers the full set.
| Nutrient class | Yields energy? | Main role | Energy value |
|---|---|---|---|
| Carbohydrates | Yes | Preferred quick fuel | 4 kcal/g |
| Proteins | Yes | Structure, enzymes, defense; last-resort fuel | 4 kcal/g |
| Lipids (fats) | Yes | Dense energy store; membranes; hormones | 9 kcal/g |
| Vitamins | No | Coenzymes and regulators | — |
| Minerals | No | Ions, bone, cofactors (Na⁺, Ca²⁺, Fe) | — |
| Water | No | Solvent, transport, temperature control | — |
Tap each nutrient class to see its role in the interactive.
- Six nutrient classes: carbohydrates, lipids, proteins (energy-yielding) and vitamins, minerals, water (no energy but essential).
- Caloric values: carbohydrate and protein 4 kcal/g, fat 9 kcal/g.
- Essential nutrients (some amino acids and fatty acids, all vitamins and minerals) must be supplied by the diet.
- Complete proteins provide all essential amino acids; complementary plant foods can be combined to do the same.
Section 5Vitamins
Tiny amounts, huge consequences
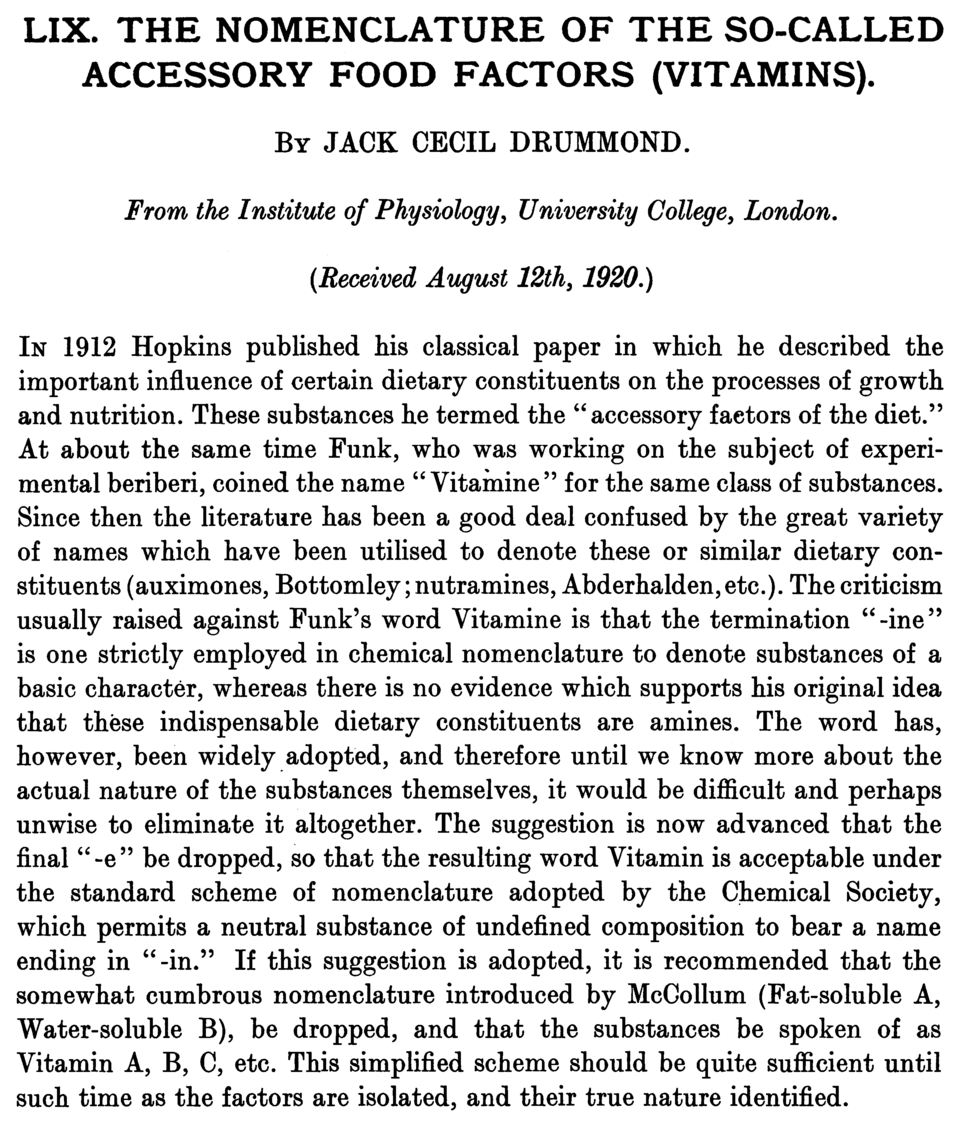
Vitamins are organic molecules the body needs in very small amounts to run its metabolism, mostly by acting as coenzymes — helper molecules that enzymes need in order to work. You need mere milligrams or micrograms a day, yet a shortfall of even one can cause a specific, sometimes deadly, deficiency disease. What makes a vitamin behave the way it does is a single physical property: how it dissolves. That splits all vitamins into two camps — fat-soluble and water-soluble — and that one fact predicts how each is absorbed, whether it is stored, and whether it can build up to toxic levels.
Fat-soluble: stored, and able to overdose
The fat-soluble vitamins are A, D, E, and K — remember them as the letters that "ADEK" up. Because they dissolve in fat, they are absorbed alongside dietary fat and then stored in the liver and fatty tissue. That storage is a double-edged sword: you can go a while without them because you have a reserve, but because the body cannot easily flush the excess, megadoses of A or D can accumulate to toxic levels. Their jobs are varied — A for vision, D for calcium balance and bone, E as an antioxidant, K for blood clotting.
Water-soluble: not stored, needed steadily
The water-soluble vitamins are the B-complex and vitamin C. Because they dissolve in water, the body does not stockpile them — any surplus is simply filtered out by the kidneys and lost in urine (which is why very high doses mostly make expensive urine). The flip side is that you need a steady daily supply, and deficiencies appear relatively quickly. Most B vitamins serve as coenzymes in energy metabolism — the very pathways from Sections 1 and 2. The classic deficiency diseases are worth knowing: scurvy from lack of vitamin C, rickets from vitamin D, beriberi from B₁, pellagra from B₃, and pernicious anemia from B₁₂.
| Property | Fat-soluble (A, D, E, K) | Water-soluble (B-complex, C) |
|---|---|---|
| Absorbed with | Dietary fat | Water |
| Stored? | Yes — liver and fat | No (B₁₂ is the exception) |
| Excess | Accumulates → toxicity risk | Excreted in urine |
| Supply needed | Less frequent (reserves exist) | Regular, near-daily |
| Deficiency example | Rickets (D), night blindness (A) | Scurvy (C), beriberi (B₁) |
Switch between the two vitamin groups and tap each one in the interactive.
- Vitamins are needed in tiny amounts and mostly act as coenzymes; solubility governs their behavior.
- Fat-soluble (A, D, E, K) are absorbed with fat, stored, and can reach toxic levels.
- Water-soluble (B-complex, C) are not stored, excess is excreted, and they need a steady daily supply.
- Each deficiency has a signature disease — scurvy (C), rickets (D), beriberi (B₁), pellagra (B₃), pernicious anemia (B₁₂).
Section 6Energy balance
A ledger, not a mystery
Body weight, at its foundation, follows a simple accounting rule called energy balance: the calories you take in as food versus the calories you spend out. When intake equals expenditure, weight holds steady (neutral balance). When intake exceeds expenditure, the surplus is stored, mostly as fat, and weight rises (positive balance). When expenditure exceeds intake, the body draws on its stores and weight falls (negative balance). The rule is straightforward; the reason weight is hard to control is that both sides of the ledger are governed by biology, not willpower alone.
Where the calories go
"Energy out" is not just exercise. Total energy expenditure has three parts. By far the largest is the basal metabolic rate (BMR) — the energy your body burns just staying alive at rest, keeping the heart beating, the kidneys filtering, and body temperature up. BMR accounts for roughly 60 to 75% of what you burn in a day, which surprises most people. A second slice, about 10%, is the thermic effect of food — the energy spent digesting and absorbing a meal. The remaining, most variable part is physical activity, from fidgeting to running a marathon. Because BMR dominates, factors that change it — muscle mass, age, thyroid hormone, body size — strongly influence how easily a person gains or loses weight.
The body defends its weight
Energy balance is not left to chance; it is regulated by the same homeostatic logic as everything else, with the hypothalamus as the control center reading hormonal signals about the body's fuel stores. Leptin, released by fat tissue, signals that stores are full and dampens appetite; ghrelin, from the empty stomach, signals hunger and stimulates eating. As a useful rule of thumb, a pound of body fat stores roughly 3,500 kcal — so a sustained deficit of about 500 kcal a day trims close to a pound a week, at least until the body adjusts its BMR downward to defend against the loss.
| Balance | Intake vs output | Result |
|---|---|---|
| Neutral | In = out | Weight stable |
| Positive | In > out | Surplus stored as fat → weight gain |
| Negative | In < out | Stores drawn down → weight loss |
Tip the balance one way or the other and see what happens in the interactive.
- Energy balance compares calories in (food) with calories out; positive balance stores fat, negative balance draws it down.
- Total expenditure = BMR (~60–75%, the largest part) + thermic effect of food (~10%) + physical activity.
- Appetite and stores are regulated by the hypothalamus using signals like leptin (full) and ghrelin (hungry).
- Roughly 3,500 kcal equals a pound of fat, but the body defends its weight by adjusting BMR.
The chapter in one breath
- Metabolism is every reaction in the body; anabolism builds and uses energy, catabolism breaks down and releases it, with ATP as the shared currency.
- Cellular respiration catabolizes glucose in four stages — glycolysis, pyruvate oxidation, the citric acid cycle, and oxidative phosphorylation — yielding up to ~32 ATP.
- Oxygen is the final electron acceptor; without it cells fall back on anaerobic fermentation for a mere 2 ATP plus lactic acid.
- The body alternates between an absorptive (store, insulin) and a postabsorptive (release, glucagon) state, with the liver keeping blood glucose steady for the brain.
- Diet supplies six nutrient classes: energy-yielding carbohydrates, lipids, and proteins (4, 9, and 4 kcal/g) plus non-energy vitamins, minerals, and water.
- Vitamins split by solubility: fat-soluble A, D, E, K are stored and can be toxic; water-soluble B and C are excreted and needed daily.
- Energy balance weighs calories in against calories out — BMR, the thermic effect of food, and activity — and the body actively defends its weight.
ReferenceWords worth knowing
A quick reference for the terms in this chapter — skim it now, or circle back whenever a word trips you up.
- Absorptive (fed) state
- The hours after a meal when nutrients are being absorbed, blood glucose rises, and the body stores surplus fuel under the direction of insulin.
- Anabolism
- The building side of metabolism — small molecules are joined into larger ones, requiring energy (endergonic).
- ATP (adenosine triphosphate)
- The cell's universal energy currency; energy is released when its terminal phosphate is removed to form ADP, and stored again when the phosphate is reattached.
- Basal metabolic rate (BMR)
- The energy the body burns at complete rest just to stay alive; the largest component of daily energy expenditure.
- Catabolism
- The breaking-down side of metabolism — large molecules are split into smaller ones, releasing energy (exergonic).
- Cellular respiration
- The controlled, stepwise catabolism of glucose that captures its energy in ATP.
- Citric acid cycle (Krebs cycle)
- The mitochondrial pathway that oxidizes acetyl CoA, releasing CO₂ and loading electron carriers (NADH, FADH₂) for the electron transport chain.
- Electron transport chain
- A series of carriers in the inner mitochondrial membrane that passes electrons to build an H⁺ gradient, powering most ATP production.
- Energy balance
- The relationship between calories taken in as food and calories expended; determines whether body weight rises, falls, or holds steady.
- Essential nutrient
- A nutrient the body cannot make in adequate amounts and therefore must obtain from the diet (certain amino acids and fatty acids, all vitamins and minerals).
- Fat-soluble vitamin
- A vitamin (A, D, E, or K) absorbed with dietary fat and stored in the body, carrying a risk of toxicity in excess.
- Gluconeogenesis
- The liver's manufacture of new glucose from non-carbohydrate sources such as amino acids, used during fasting.
- Glycogenolysis
- The breakdown of stored glycogen back into glucose to raise blood sugar between meals.
- Glycolysis
- The first stage of respiration, in the cytoplasm, splitting glucose into two pyruvate and netting 2 ATP without oxygen.
- Ketone bodies
- Acidic fuel molecules made by the liver from fat during prolonged fasting; usable by the brain but able to lower blood pH.
- Kilocalorie (Calorie)
- The unit of food energy; carbohydrate and protein yield ~4 kcal/g, fat ~9 kcal/g.
- Metabolism
- The sum of all chemical reactions in the body, comprising anabolism and catabolism.
- Oxidative phosphorylation
- The final stage of respiration on the inner mitochondrial membrane, using the electron transport chain and oxygen to generate the bulk of ATP.
- Postabsorptive (fasting) state
- The period between meals when stored fuel is released to maintain blood glucose, directed by glucagon.
- Vitamin
- An organic molecule required in tiny amounts, usually acting as a coenzyme in metabolism.
- Water-soluble vitamin
- A vitamin (the B-complex or C) that dissolves in water, is not stored, is excreted in excess, and must be supplied regularly.